All published articles of this journal are available on ScienceDirect.
Abiotic Stress-induced Changes in Bioactive Compounds of Fruit Crops: A Review
 iD
Obadiah A.2
iD
Jeevitha D.1
iD
Matheshwaran1
iD
Giriprasath R. S.1
iD
A. Bharanidharan1
iD
Authors Info & Affiliations
Abstract
Introduction
Abiotic stress is one of the major constraints limiting crop productivity, plant growth, and fruit quality worldwide. Environmental stresses such as drought, salinity, temperature extremes, heavy metals, and oxidative stress adversely affect plant metabolism, development, and survival.
Materials and Methods
This review synthesizes published literature on the role of plant secondary metabolites in mediating tolerance to major abiotic stresses. Particular emphasis is placed on the functions of terpenes, phenolic compounds, and nitrogen-containing compounds in plant stress adaptation. Nitrogen-containing compounds have greater effects against biotic stress than abiotic stress.
Results
The reviewed studies indicate that secondary metabolites play significant roles in mitigating abiotic stress. Phenolic compounds, particularly flavonoids and stilbenes, function as powerful antioxidants and photoprotective agents, while terpenes contribute to cellular stability under stress conditions. Nitrogen-containing metabolites, including alkaloids, glucosinolates, and cyanogenic glycosides, also participate in defence responses and stress tolerance. Collectively, these compounds contribute to Reactive Oxygen Species (ROS) scavenging, antioxidant activity, osmotic regulation, membrane stability, and stress signalling pathways.
Discussion
The findings highlight the diverse mechanisms through which secondary metabolites enhance plant resilience to environmental stresses. Their accumulation and activity are critical components of plant adaptive responses and may influence stress tolerance across different crop species and stress conditions.
Conclusion
Secondary metabolites play a crucial role in enhancing plant adaptation to adverse environmental conditions. A better understanding of their mechanisms of action may facilitate the development of stress-resilient crops and support sustainable agricultural production under changing climatic conditions.
1. INTRODUCTION
Plants are continuously exposed to changing environmental conditions that influence their growth, development, and productivity. Unlike animals, plants are unable to escape adverse environmental conditions because of their sessile nature [1]. Plants inhabit dynamic environments that are frequently detrimental to their growth and development [2]. In addition to their ecological role in capturing solar energy, absorbing atmospheric CO2, and producing oxygen and organic matter, plants provide fruits that are important sources of bioactive compounds with nutritional and health-promoting properties. Abiotic stresses are major environmental factors influencing plant productivity and distribution. Unfavourable environmental conditions, including drought, heat, cold, nutrient deficiencies, salinity, and toxic metal accumulation in soils, pose a continual threat to plant growth and agricultural production [3]. These stresses reduce the amount of arable land available globally and negatively affect crop yield, quality, survival, adaptability, and lifespan [4]. Extreme weather events can result in severe crop losses, while chronic abiotic stress can limit crop cultivation across large geographic regions [5]. Consequently, abiotic stresses have significant implications for food security, national economies, and the livelihoods of farming communities [6]. In plants, stress refers to any environmental condition that disrupts normal growth, development, metabolism, or productivity [7]. Beyond their effects on growth and yield, abiotic stresses can also influence the synthesis and accumulation of secondary metabolites, including phenolics, flavonoids, carotenoids, and anthocyanins. These bioactive compounds play important roles in plant defence mechanisms and contribute to the nutritional, sensory, and functional quality of fruits. In some cases, moderate stress conditions may enhance the accumulation of health-promoting phytochemicals, whereas severe stress may adversely affect fruit quality and productivity. Although numerous studies have investigated plant responses to individual abiotic stresses, a comprehensive synthesis of their effects on bioactive compound accumulation and fruit nutritional quality remains limited. Furthermore, the dual role of abiotic stress as both a constraint to crop production and a potential inducer of beneficial phytochemicals has not been adequately summarized across fruit crops. Therefore, this review aims to critically examine the effects of major abiotic stresses on fruit crops, with particular emphasis on stress-induced changes in bioactive compounds, physiological responses, and fruit quality attributes. The literature included in this review was retrieved from major scientific databases, including Google Scholar, Scopus, Web of Science, and PubMed. Relevant peer-reviewed research articles, review papers, books, and book chapters published primarily between 2000 and 2025, along with selected seminal studies, were identified using keywords such as “abiotic stress”, “flavonoids”, “terpenoids”, “Osmoprotectants”, “phytochemicals”, “reactive oxygen species (ROS)”, and “fruit crops”. Studies focusing on the role of secondary metabolites in abiotic stress tolerance and stress-induced changes in fruit were critically evaluated in this review.
2. ABIOTIC STRESS
Any unfavorable environmental factor that prevents a plant from growing properly is referred to as abiotic stress [8-10]. Crop productivity, lifespan, survival, health, and adaptability were all negatively affected by abiotic factors [5]. Heat, cold, drought, flood, salinity, and heavy metal stress are the categories into which it can be divided (Fig. 1).
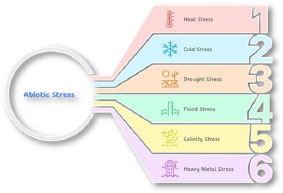
Types of abiotic stress.
2.1. Heat Stress
The timing of biological processes and, consequently, the growth and development of living biota are significantly influenced by temperature. The heat unit system, also known as Growing Degree Days (GDDs), is predicated on the idea that temperature and plant development are generally directly and linearly correlated. A “Growing Degree-Day” (GDD) is a common way to represent the amount of heat energy an organism collects over time. GDD accumulation during the day is necessary for biomass production, while GDD accumulation during the night is necessary for flower formation. Heat units, often called “growing degree days,” are a method of assigning each day a heat value. The heat units of fruit crops are presented in Table 1. These heat units describe the optimal requirements needed for maturity, and values above these can lead to heat stress. Tropical crops typically have higher threshold temperatures, while temperate crops typically have lower values.
| S.no | Fruits | Cultivar | Base Temperature | Heat Units for Maturity |
|---|---|---|---|---|
| 1 | Mango | Kesar | 17.9ºC | 780-796 |
| Banganapalli | 18ºC | 1426-1445 | ||
| 2 | Banana | - | 9.8ºC | 1930 |
| 3 | Ber | Gola | 7.2ºC | 1980-2236 |
| Kaithali | 7.2ºC | 2236-2566 | ||
| Umran | 7.2ºC | 2290-2516 | ||
| 4 | Litchi | Shai | 15ºC | 813 |
| 5 | Citrus | - | 13ºC | 1600-1900 |
| 6 | Papaya | - | 12ºC | 2000 |
| 7 | Pecan Nuts | - | 10ºC | 2700-3000 |
Heat units are used to determine whether a location is suitable for growing a specific crop, estimate the amount of heat stress on crops, and forecast the dates of physiological maturity and harvest. The effects of heat stress on bioactive compounds vary among fruit crops depending on stress intensity, duration, genotype, and developmental stage. Moderate heat stress may stimulate the production of Reactive Oxygen Species (ROS), activating antioxidant defence mechanisms and the phenylpropanoid pathway, thereby increasing the accumulation of phenolics, flavonoids, and anthocyanins in some crops such as strawberry. In contrast, excessive temperatures during fruit development and ripening may inhibit anthocyanin biosynthesis and promote pigment degradation, as reported in grapes, resulting in reduced fruit coloration and antioxidant capacity.
| S.no | Crop | Impact | References |
|---|---|---|---|
| 1. | Mango | • Highest percentage of necrotic symptoms – Bombay Green and Himsagar. • Difference in phenolic compounds between affected and non-affected fruits |
[11] |
| 2. | Grapes | • Positive Effect – Sugar Accumulation • Negative effect – Anthocyanin Biosynthesis |
[12] |
| 3. | Citrus | • Carotenoid Content – Decreases with the increase in temperature | [13] |
| 4. | Strawberry | • Total phenolics, total flavonoids, and anthocyanin increase with the rise in temperature | [14] |
2.2. Cold Stress
To synchronize flowering, fruit crops require chilling, or a cold period during winter. Inadequate chilling may induce uneven, irregular, delayed flowering, leading to a high rate of floral abortion [15]. Asynchronous fertilization and pollination could result from this, which would reduce fruit set and production [15]. Table 3 presents the chilling requirement of fruit crops.
| Fruit Crops | Chilling Hours |
|---|---|
| Citrus | 0-100 CH |
| Grapes | 100-200 CH |
| Fig | 100-500 CH |
| BlackBerry | 200-500 CH |
| Japanese Plum | 300-500 CH |
| Almond | 500-600 CH |
| Apricot | 400-750 CH |
| Peach | 500-800 CH |
| Kiwi | 600-800 CH |
| European Plum | 500-900 CH |
| Apple | 1300 CH |
Understanding the required chilling hours is essential for choosing fruit crops and cultivars appropriate to particular agroclimatic zones, especially as the climate changes. Chilling requirement should be distinguished from cold stress. Agroclimatic zones refer to regions with similar climatic and edaphic conditions that influence crop growth, productivity, and management practices. Chilling requirement refers to the exposure of dormant buds to a specific duration of low temperatures necessary for normal bud break, flowering, and fruit set. In contrast, chilling injury occurs when plants are exposed to low, non-freezing temperatures that disrupt physiological processes, while freezing stress results from temperatures below the freezing point, leading to ice crystal formation and cellular damage. Membrane damage and ion leakage, cell dehydration from ice crystal formation, protein structure and stability disruption, decreased antioxidant enzyme activity, ROS production and lipid peroxidation, altered signalling and gene expression, decreased photosynthetic rate, decreased plant growth and weight, inhibited seed germination, and decreased agricultural production are all effects of cold stress on plants [16]. Plant responses to cold stress include changes in cell membrane fluidity, the expression of cold resistance genes, overcoming cellular dehydration, enhancing antioxidant systems, limiting the production of ROS and MDA, increasing photosynthetic rate, increasing the synthesis of osmoprotectants, improving growth parameters, improving seed germination, and adapting the phenological cycle to an ideal term [16]. It also has an impact on bioactive compounds of fruit crops, as provided in Table 4.
| S.no | Crop | Impact | References |
|---|---|---|---|
| 1. | Mango | Flavonoid, Anthocyanin Level – Decrease with Low Temperature | [17] |
| 2. | Strawberry | Freezing Temperature (-10ºC) – Increase in phenolics over control | [18] |
| 3. | Grapes | Low Temperature (10/7ºC) – Decrease in Phenolic Compounds | [19] |
| 4. | Banana | Total phenolic compounds – Increase with increase in duration of time | [20] |
2.3. Drought Stress
Drought stress is one of the major abiotic factors limiting the growth, productivity, and fruit quality of horticultural crops. The annual water requirement of fruit crops, as shown in Tables 5 and 6, demonstrates that the environment and growth patterns of various fruit crops determine the amount of water they need. Drought stress occurs when water availability becomes insufficient to support normal physiological and metabolic processes throughout the plant life cycle [21, 22]. Under drought conditions, plants experience oxidative stress due to excessive accumulation of Reactive Oxygen Species (ROS), leading to cellular damage, reduced photosynthesis, impaired pigment synthesis, and altered hormonal signalling pathways involving Abscisic Acid (ABA), ethylene, and Jasmonic Acid (JA) [23].
| Fruit Crops | Rainfall (mm) |
|---|---|
| Banana | 1200-2200 |
| Citrus | 900-1200 |
| Grapes | 500-1200 |
| Pineapple | 700-1000 |
| Fruit Crops | Water Requirement |
|---|---|
| Mango | 30-40 (litres/plant/day) |
| Guava | 22-30 (litres/plant/day) |
| Banana | 8-12 (litres/plant/day) |
| Sapota | 30-40 (litres/plant/day) |
| Grapes | 10-15 (litres/plant/day) |
To counteract these adverse effects, plants activate various defence mechanisms, including the enhanced biosynthesis of secondary metabolites such as phenolics, flavonoids, terpenes, and other antioxidant compounds. These bioactive compounds function as ROS scavengers, osmoprotectants, and stress signalling molecules that help maintain cellular homeostasis and membrane stability under water-deficit conditions. In several fruit crops, drought stress has been associated with increased accumulation of phenolic compounds, anthocyanins, and flavonoids, thereby enhancing antioxidant capacity and stress tolerance (Table 7).
| S.no | Crop | Impact | References |
|---|---|---|---|
| 1. | Papaya | Non-irrigated plants– increase in Phenolic Compounds. | [24] |
| 2. | Apple | Total Phenolics – Increase in Cultivars after 12 days. | [25] |
| 3. | Apple | Anthocyanin – Increases with the increase in drought stress. | [26] |
| 4. | Fig | Anthocyanin – Higher in drought compared to watered. | [27] |
2.4. Flood Stress
Fruit crops that are susceptible to moist conditions may experience a number of negative effects from flooding or waterlogging conditions in the soil. The susceptibility of plants to flood conditions affects their growth and output [28]. Flooding is characterized by an excess of water caused by heavy or unexpected rainfall and inadequate drainage, which stresses vegetation [28]. In wet soil, oxygen partial pressure and gas diffusion steadily decrease, interfering with normal cellular functions and metabolism as well as plant root function. One major element restricting crop growth and productivity is waterlogging [29]. Anoxic conditions, decreased root hydraulic conductivity, decreased biosynthesis and increased chlorophyll breakdown, decreased photosynthetic activity, and decreased stomatal conductance are all consequences of flood stress on plants [30], and in fruit crops, the impacts are listed in Table 8. Flooding-induced hypoxia or anoxia disrupts normal metabolic processes and promotes the generation of Reactive Oxygen Species (ROS), leading to changes in antioxidant defence systems. As a stress response, the activities of antioxidant enzymes such as Superoxide Dismutase (SOD), Catalase (CAT), and Peroxidase (POD) may increase, along with alterations in the accumulation of phenolics and flavonoids. However, prolonged flooding can impair carotenoid biosynthesis, shift metabolism toward anaerobic pathways, and reduce fruit quality by affecting nutritional composition, color development, and antioxidant potential.
| S.no | Crop | Impact | References |
|---|---|---|---|
| 1. | Banana | The air circulation in roots is absent for the normal respiration process. Therefore, the plants show yellowing symptoms, and severe stages result in death. | [31] |
| 2. | Peach | Reduction of the root hydraulic conductivity. | [32] |
| 3. | Passion fruit | 7, 14, and 21 days of flooding - the carotenoid level was higher in seedlings. | [33] |
2.5. Salinity Stress
One of the main environmental stressors that restricts plant development and productivity is salinity. 7% of the land is made up of saline soils [34]. EC of different fruit crops are listed in Table 9. Excessive concentrations of soluble salts that impede or interfere with normal plant growth processes are known as salinity. Electrical Conductivity (EC), Exchangeable Sodium Percentage (ESP) or Sodium Adsorption Ratio (SAR), and the pH of a saturated soil are used to measure it. A soil is considered saline if its pH is less than 8.5, its EC is greater than 4 dS m–1, and its ESP is less than 15% [35-38]. Chloride, sulphate, sodium, magnesium, and calcium ions are mixed with sodium chloride in saline soils.
| Fruit Crops | Threshold EC (ds/m) |
|---|---|
| Almond | 1.5 |
| Apricot | 1.6 |
| Blackberry | 1.5 |
| Date palm | 4.0 |
| Grapes | 1.5 |
| Grapefruit | 1.2 |
| Guava | 4.7 |
| Lemon | 1.5 |
| Sweet orange | 1.3 |
| Peach | 1.7 |
| Plum | 2.8 |
Salinity stress causes non-toxic compatible solute accumulation, osmotic stress- or abscisic acid-induced stomatal closure, programmed cell death under extreme salinity shock, browning and death of leaves, abscisic acid formation in roots and stems followed by its transport to the leaves, leading to low water uptake efficiency, poor root growth, and high Na and Cl accumulation in roots, which competes with the uptake of Ca, Zn, P, and NO2 [39]. Salinity stress also affects the bioactive compounds of fruit crops (Table 10). Salinity-induced oxidative stress stimulates the generation of Reactive Oxygen Species (ROS), which activate antioxidant defense mechanisms and the phenylpropanoid pathway, leading to increased synthesis of phenolic compounds and flavonoids. These metabolites help plants mitigate oxidative damage and maintain cellular homeostasis under moderate salinity stress. However, at higher salinity levels, severe osmotic stress and ion toxicity impair photosynthesis, nutrient uptake, and carbon assimilation, resulting in reduced plant growth, fruit yield, and, in some cases, decreased accumulation of beneficial bioactive compounds.
| S.no | Crops | Impact | References |
|---|---|---|---|
| 1. | Banana | • In vitro Culture – Phenolic increases till 100 mM NaCl. | [40] |
| 2. | Strawberry | • There is an increase in total phenols and flavonoids with an increase in salinity. | [41] |
| 3. | Grapes | • Salinity (50 mM) – Raised the phenolic concentration in both roots and leaves | [42] |
| 4. | Pomegranate | • There is an increase in phenolics and flavonoids from (0 to 75 mM) and differs for different cultivars. | [43] |
2.6. Heavy Metal Stress
Abiotic and biotic stressors are a constant for plants in the natural world. For a long time, anthropogenic processes like industrial waste, fertilizer applications, smelting, and sewage disposal have caused heavy metals like Fe, Mn, Cu, Ni, Co, Cd, Zn, Hg, and arsenic to build up in soils [44]. Metal-related abiotic stress in fruit crops includes both excess accumulation of essential micronutrients and exposure to non-essential toxic metals. Essential micronutrients such as Cu, Fe, Mn, Zn, and Ni are required for normal physiological and biochemical functions in plants; however, excessive accumulation of these micronutrients can induce oxidative stress and metabolic disturbances. In contrast, non-essential toxic metals such as Cd, Pb, Hg, and As have no known biological function and are highly toxic even at low concentrations, adversely affecting plant growth, fruit quality, and food safety. While several of these metals are essential micronutrients for many typical plant functions, excess can be harmful and directly affect plant development, metabolism, physiology, and senescence. Heavy metals have negative effects on plant growth and development, including decreased plant production and quality, disruption of the flowering cycle, yellowing, drying, and senescence of leaves, suppression of stem branch growth, inhibition of root growth and elongation, root atrophy and even death, and a decrease in the germination rate of plant seeds. Impacts of fruit crops due to heavy metal stress are listed in Table 11. In addition to affecting plant growth, heavy metal stress can modify the accumulation of bioactive compounds in fruits. Moderate levels of metal-induced oxidative stress may enhance the synthesis of phenolics, flavonoids, and other antioxidant metabolites as part of the plant defence response. However, prolonged or severe exposure can disrupt metabolic pathways, reducing phytochemical accumulation and fruit nutritional quality. Furthermore, the accumulation of toxic metals in edible tissues raises food-safety concerns due to potential risks to human health. Heavy metals limit peroxidation of cell membranes, which in turn affects SOD, CAT, POD, APX, NR, GR, and other physiological and ecological traits of plants. They also reduce chlorophyll content and photosynthetic efficiency, repress plant nitrogen metabolism, respiration, and nucleic acid metabolism, increase protein solubility and proline content, and inhibit plant nutrient absorption and transport [45].
| S.no | Crop | Impact | References |
|---|---|---|---|
| 1. | Pineapple | The root elongation and biomass of Tainung No. 17 were affected negatively by 300 µM AlCl3. | [46] |
| 2. | Plum | Natural cadmium content (plants) - 0.02 to 0.50 mg/kg of dry matter. The concentration of cadmium in fruit exceeded the natural value of 0.8 mg/kg | [47] |
| 3. | Citrus | The highest level of total flavonoid concentration was measured at 500 µM Cu concentration. The highest phenol concentration was recorded at 500 µM Pb + Cu compared to the control. | [48] |
3. SECONDARY METABOLITES
A wide variety of chemical molecules that are not directly involved in plant growth and development are produced by plants. These compounds are referred to as natural products, secondary products, or secondary metabolites. In particular, while primary metabolites are present across the plant kingdom, secondary metabolites are sometimes limited to a single plant species or closely related group of species. Amino acids, sugars, nucleotides, and other substances are examples of primary metabolites [49].
3.1. Bioactive Compounds: Sources and Definitions
Secondary plant metabolites have toxicological or pharmacological effects on both humans and animals. Even though certain nutrients, such as vitamins and minerals, can have pharmacological or toxicological effects when consumed in large quantities, they are typically not part of the bioactive plant chemical.
3.2. Classification of Secondary Metabolites
The secondary metabolites can be classified into terpenes, phenolics, and nitrogen-containing compounds in Fig. (2).
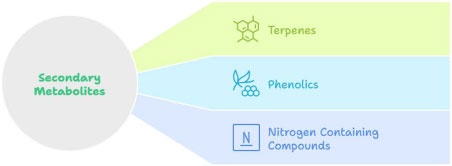
Three major classifications of secondary metabolites.
3.3. Pathways of Secondary Metabolites
Different pathways of secondary metabolites are listed in Table 12. The link between primary and secondary carbon metabolism in plants shows how complex secondary metabolites begin with simple carbon molecules produced during photosynthesis. Phosphoenolpyruvate (PEP), pyruvate, 3-Phosphoglycerate (3-PGA), erythrose-4-phosphate, and other key intermediates are produced when carbon dioxide fixed by photosynthesis enters primary carbon metabolism. The Tricarboxylic Acid (TCA) cycle, which produces aliphatic amino acids, and the transformation of pyruvate into acetyl-CoA, a significant metabolic hub, are two important routes into which these molecules move. Different kinds of secondary metabolites are produced by specialized biosynthetic pathways that diverge from these main processes. The shikimic acid pathway, fed by erythrose-4-phosphate and PEP, generates aromatic amino acids such as phenylalanine and tyrosine, which then yield secondary metabolites containing nitrogen and a variety of phenolic compounds. The malonic acid pathway contributes to the generation of phenolic compounds through a series of condensation reactions. Acetyl-CoA enters the mevalonic acid pathway to produce isoprenoid units, which lead to the synthesis of different terpenes, but the MEP (methylerythritol phosphate) pathway, which begins with 3-PGA and pyruvate, provides an alternative route for terpene production. Together, these pathways demonstrate how basic carbon intermediates from primary metabolism are intricately transformed into structurally diverse and biologically significant secondary metabolites, such as terpenes, phenolics, and nitrogen-containing compounds, all of which are essential for plant Défense, signalling, pigmentation, and environmental adaptation [49].
| Compound | Originating Pathways |
|---|---|
| Erythrose-4-Phosphate | Pentose Phosphate Pathway |
| Phosphoenolpyruvate | Glycolysis Pathway |
| Pyruvate | Glycolysis Pathway |
| 3-Phosphoglycerate (3-PGA) | Calvin or C3 Cycle |
3.4. Mechanism of Bioactive Compounds Accumulation due to Abiotic Stress
Plants respond to a range of abiotic stimuli, such as drought, salinity, nutritional deficiencies, extreme temperatures, heavy metals, and intense light, by activating complex physiological, biochemical, and molecular defense systems. Increased production of phenolic compounds and enhanced tolerance to oxidative stress are the end results of these pathways. When a plant experiences environmental stress, Reactive Oxygen Species (ROS) rapidly accumulate in a number of organelles, such as mitochondria and chloroplasts. These ROS serve as early signalling molecules in plant cells, initiating calcium-dependent pathways and MAPK (mitogen-activated protein kinase) cascades. Significant gene expression reprogramming occurs when these intracellular signals are triggered, allowing the plant to begin defensive metabolic changes. One significant reaction is the oxidative pentose phosphate pathway, which generates NADPH, an essential reducing agent required for both biosynthesis and antioxidant defense. The major enzyme that initiates the phenylpropanoid pathway, Phenylalanine Ammonia Lyase (PAL), becomes more active when the shikimate pathway is simultaneously activated by NADPH and stress signals. This system produces a variety of phenolic compounds, such as flavonoids, phenolic acids, tannins, and lignin precursors. Proline, which serves as an osmolyte to protect cellular structures and aid in the detoxification of Reactive Oxygen Species (ROS), also accumulates under stress [50]. Increased activity of antioxidant enzymes, participation in intercellular stress communication including ABA, Ca2+, and ethylene, and enhanced photosynthetic efficiency by preserving chloroplast function under stress are only a few of the defensive roles supported by the rise in phenolic compounds. Furthermore, phenolics regulate the synthesis of other secondary metabolites that bolster the plant's defensive system. As ROS levels fall and antioxidant capacity rises, oxidative stress is successfully reduced and systemic acquired resistance is strengthened through Salicylic Acid (SA) signalling and activation of the NPR1 regulatory protein. These interconnected pathways demonstrate how plants integrate metabolic, hormonal, and molecular responses to lessen abiotic stress and maintain cellular homeostasis by boosting the accumulation of phenolic compounds and other protective metabolites [50].
3.5. Role of Secondary Plant Metabolites
They protect plants against herbivory (being eaten by herbivores) and against infection by microbial pathogens [49]. Secondary metabolites from plants are important sources of flavours, food additives, medications, and pharmaceuticals, with significant industrial use [59], and they differ among fruit crops (Table 13). These substances influence ecological interactions, such as attracting parasitic wasps to manage pest populations, in addition to providing protection against direct dangers [60].
| Fruits | Classification | Compound | References |
|---|---|---|---|
| Mango | Terpene (Tetraterpene) | Beta Carotene | [51] |
| Grapes | Stilbenes | Resveratrol | [52] |
| Almond | Cyanogenic Glucosides | Amygdalin | [53] |
| Peach | Cyanogenic Glucosides | Prunasin | [54] |
| Citrus | Terpene (Monoterpene) | Limonene | [55] |
| Grapes | Flavanols | Catechin | [56] |
| Citrus | Flavanone | Hesperidin, Naringenin | [57] |
| Pomegranate | Hydrolyzable Tannin | Punicalagin | [58] |
3.6. Terpenes
They are insoluble in water and belong to the largest class of secondary metabolites. Acetyl-CoA or glycolytic intermediates are used in their biosynthesis. The union of five-carbon atoms with the branching carbon skeleton of isopentane is the source of all terpenes (Fig. 3). Because terpenes can break down into isoprene units at high temperatures, the fundamental structural components of terpenes are frequently referred to as isoprene units. It is sometimes referred to as isoprenoids [49]. Classification of Terpenoids is presented in Fig. (4) and Table 14.
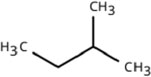
Structure of isopentane.
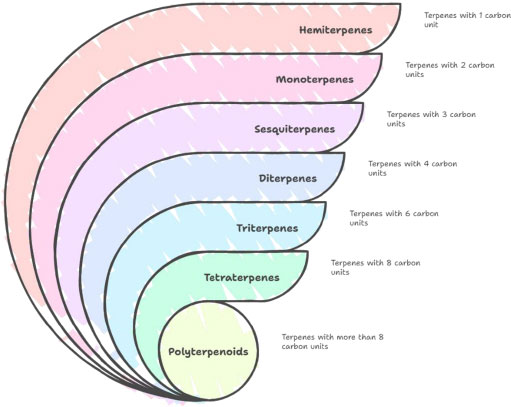
Classification of terpenoids.
| S.no | Type of Terpenes | Compound | Structure | Source | Methodology | References |
|---|---|---|---|---|---|---|
| 1. | Hemiterpenes (C5H8) |
Isovaleric acid | 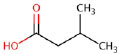 |
Jack fruit | HPLC | [61] |
| 2. | Monoterpenes (C10H16) |
Linalool | 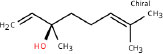 |
Guava, Sweet Orange | GC-O | [62] |
| Citronellol | 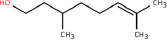 |
Lime, Lemons, Oranges, Grapefruit | GC-MS | [63] | ||
| Thymol | 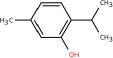 |
Thyme plant (Thymus vulgaris) |
GC-MS | [64] | ||
| Carvacrol | 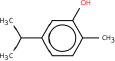 |
Oregano (Origanum Vulgare) |
GC-MS | [65] | ||
| 3. | Sesquiterpenes (C15H24) |
Curcumenol | 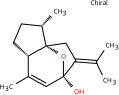 |
Curcuma sp. | GC-MS | [66] |
| Artelinic acid | 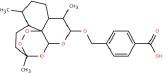 |
Artemisia annua | GC-MS | [67] | ||
| 4. | Diterpenes (C20H32) |
Steviol | 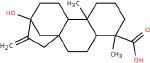 |
Stevia (Stevia rabaudiana) |
HPLC | [68] |
| Carnosic acid | 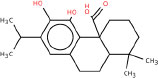 |
Rosemary (Rosmarinus officinalis) |
HPLC | [69] | ||
| 5. | Triterpenes (C30H48) |
Sitosterol | 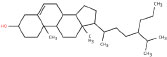 |
Avocado, Banana. | GC-MS | [70] |
| Stigmasterol | 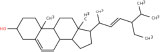 |
Passion fruit, Avocado | GC-MS | [70] | ||
| 6. | Tetraterpenes (C40H64) |
Beta-Carotene | 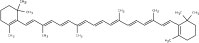 |
Mango, Papaya | HPLC | [51] |
| Lutein | 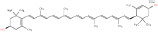 |
Kiwi, Oranges | HPLC-UV | [71] |
3.6.1. Examples of Terpenes Based on the Classification
3.6.1.1. Biosynthesis of Terpenoids
The biosynthesis of terpenoids consists of two major pathways: the Mevalonate and the methylerythritol pathways. The two main metabolic pathways that produce the necessary five-carbon precursors, Isopentenyl Diphosphate (IPP) and Dimethylallyl Diphosphate (DMAPP), are the Mevalonate (MVA) pathway and the Methylerythritol Phosphate (MEP) pathway. Figure 6 shows the full biosynthesis of isoprenoids (terpenoids). Three acetyl-CoA molecules condense in the MVA pathway to form mevalonic acid, which is then phosphorylated and decarboxylated to yield IPP. IPP and DMAPP can be interconverted as needed. Glyceraldehyde-3-phosphate and pyruvate combine to make methylerythritol phosphate in the MEP pathway, which is then subjected to many enzymatic processes to yield the identical IPP and DMAPP precursors. Then, these two five-carbon units function as universal building blocks for terpenoids that get bigger with time: Geranyl diphosphate (GPP, C11), the precursor of monoterpenes, is formed when IPP and DMAPP combine; farnesyl diphosphate (FPP, C1) is formed when another IPP is added, resulting in sesquiterpenes (C1) and triterpenes (C30); and geranylgeranyl diphosphate (GGPP, C20), the precursor for diterpenes (C20), tetraterpenes (C40), and larger polyterpenoids. Overall, the image illustrates how two distinct yet convergent pathways convert simple carbon substrates into a wide variety of terpenoid compounds that are essential to plant defence, metabolism, signalling, colour, and cellular structure [49].
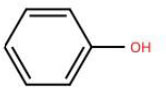
Structure of phenolic compounds.
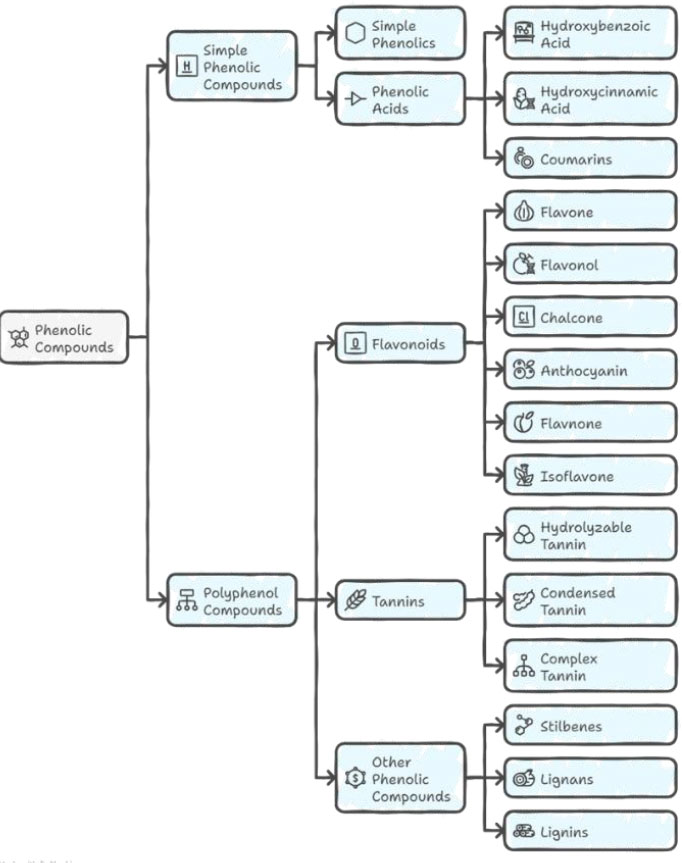
Classification of phenolic compounds.
3.6.2. Role of Terpenes in Abiotic Stress
Increased levels of different terpenes in fruit crops are listed in Table 15. Terpenes reduce oxidative stress in abiotic stress by two mechanisms: (i) direct intercellular reactions with oxidants or (ii) modification of ROS signalling. Terpenes have crucial functions in membrane stability and antioxidant actions [72]. This involves ROS Scavenging, membrane stabilization, and hormone signalling [73].
3.7. Phenolic Compounds
The majority of vegetable-based foods contain phenolic compounds, which are a variety of families of compounds that are widely distributed in nature. They include thousands of different chemicals, ranging from simple phenolic acids to complex flavonoids. These substances have attracted significant interest due to their impact on several organoleptic characteristics, such as taste and colour. A hydroxyl functional group on an aromatic ring is called a phenol group (Fig. 5). They are a collection of almost 10,000 distinct chemicals that are chemically diverse [49]. In nature, they is everywhere. They are recognized to have anti-inflammatory, antibacterial, and antioxidant properties [76]. Phenolic compounds are classified as in Fig. (6) and Table 16. Anthocyanins can be further divided into many types as presented in Fig. (7). Sources of various phenolic compounds of different crops are listed in Table 17.
| S.no | Classification | Structure | Description |
|---|---|---|---|
| 1. | Simple Phenolic Compounds |
 |
It contains one phenol unit and is considered Simple. |
| 2. | Hydroxybenzoic acid |
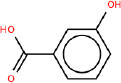 |
The carboxylic acid functional group is directly bonded to the phenol ring. |
| 3. | Hydroxycinnamic acid |
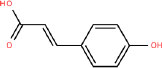 |
The carboxylic acid functional group and the phenol ring are separated by two doubly bonded carbons. |
| 4. | Coumarins |
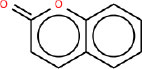 |
A benzene ring fused to an alpha-pyrone ring, a six-membered ring containing one oxygen atom and a carbonyl group (ketone). |
| 5. | Flavonoids |
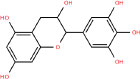 |
A and C are either mono-, di-, or trihydroxylated. |
| 6. | Hydrolysable Tannin |
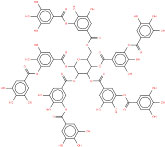 |
Gallotannins or ellagitannins. Gallotannins are polyols that are substituted with gallic acid units. Commonly, the polyol core is a D-glucose, and galloyl units in gallotannins are linked by depside (ester) linkages. |
| 7. | Condensed Tannins |
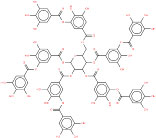 |
Polymeric phenolic compounds that consist of catechin units. When depolymerized, they give anthocyanidin. Thus, condensed tannins are called proanthocyanidins. |
| 8. | Complex Tannins | 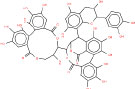 |
Gallotannins or ellagitannins bonded to a catechin unit. |
| 9. | Stilbenes | 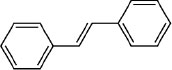 |
Stilbenes are phenolic compounds in which two phenol units are linked by two doubly bonded carbons. |
| 10. | Lignan | 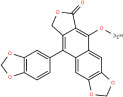 |
Consists of two phenol units linked by four carbons. |
| 11. | Lignin | 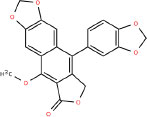 |
Consists of phenol units or phenolic compounds that are linked with each other by carbon chains. It has high molecular weight. |
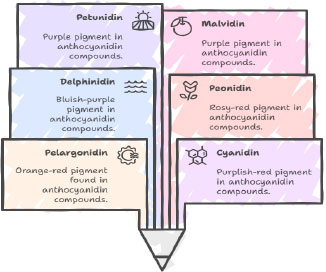
Types of anthocyanidins.
| S.no | Type of Phenolic Compounds | Derivatives | Structure | Source | Methodology | References |
|---|---|---|---|---|---|---|
| 1. | Flavones | Luteolin | 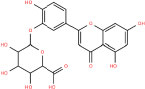 |
Apple, pear, peach | HPLC-LC/DAD | [77] |
| Apigenin | 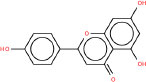 |
Oranges, strawberries | HPLC-LC | [78] | ||
| 2. | Isoflavones | Daidzein | 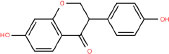 |
Peaches, plums | GC-MS | [79] |
| Genistein | 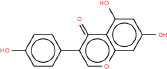 |
Sour cherry | HPLC-MS | [80] | ||
| 3. | Flavanols | (+)-Catechin | 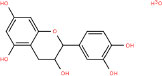 |
Grapes, apple | HPLC | [81] |
| (-)- Epicatechin |
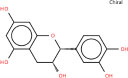 |
Pear, grapes |
HPLC | [81] | ||
| Quercetin | 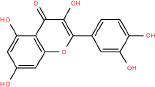 |
Grapes, citrus |
HPLC | [82] | ||
| Kaempferol | 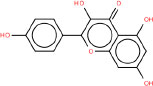 |
Peaches, black berries |
HPLC | [82] | ||
| Myricetin | 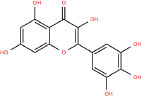 |
Cranberry, blueberry |
HPLC | [82] | ||
| 4. | Flavanones | Hesperidin | 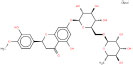 |
Citrus | UV-vis | [83] |
| Naringenin | 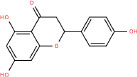 |
Citrus | UV-vis | [83] | ||
| 5. | Chalcone | Phloretin | 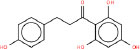 |
Apple, pear |
HPLC-DAD -MS/MS |
[84] |
| 6. | Stilbenes | Resveratrol | 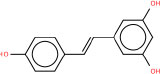 |
Grapes | HPLC | [85] |
3.7.1. Biosynthesis of Phenolic Compounds
The phenylpropanoid and flavonoid biosynthesis pathway in plants produces numerous significant secondary metabolites. The route starts with the amino acid phenylalanine, which is converted to trans-cinnamic acid by the enzyme Phenylalanine Ammonia-Lyase (PAL). P-coumaric acid, a crucial branching point in phenylpropanoid metabolism, is created by further modifying this molecule, which acts as a central intermediate. Plants produce a number of classes of chemicals from p-coumaric acid, such as derivatives of benzoic acid, caffeic acid, and other simple phenylpropanoids, coumarins, and precursors of lignin, all of which are vital for plant defense and structure. Chalcone synthase transforms p-coumaric acid into p-coumaroyl-CoA, which subsequently combines with three molecules of malonyl-CoA to produce chalcones. The initial committed intermediates in the production of flavonoids are chalcones. These substances are then transformed into flavanones, which serve as key intermediates in the synthesis of various flavonoids. Anthocyanins and condensed tannins are the final products of the further transformation of flavanones into flavones, isoflavones, flavonols, and dihydroflavonols. Plant pigmentation, antioxidant activity, UV protection, and disease resistance are all influenced by these metabolites [49].
3.7.2. Regulation of Flavonoids Under Cold Stress
The combined physiological and molecular responses of plants to cold stress are depicted in Fig. (8), with a focus on membrane stability, transcriptional control, regulation of Reactive Oxygen Species (ROS), and flavonoid accumulation. One significant abiotic stressor that disrupts cellular homeostasis is cold stress, which primarily affects membrane integrity and metabolic functions. One of the main locations of cold perception is the cell membrane, which is altered at the cellular level when exposed to low temperatures. By altering the lipid composition of their cell membranes, plants improve their fluidity and stability in response to cold-induced stiffness. This adaptive modification helps to preserve membrane function and prevents cellular contents from escaping. However, cold stress also leads to an excess of Reactive Oxygen Species (ROS), such as hydrogen peroxide (H2O2) and superoxide radicals (O2−). This coordinated enzymatic action maintains the balance of ROS. Electrolyte Leakage (EL) and Malondialdehyde (MDA), two indicators of oxidative stress, are consequently reduced, suggesting improved cellular integrity and reduced membrane lipid peroxidation. At the same time, Proline (PRO), an Osmoprotectant that helps stabilize proteins and membranes under cold conditions, increases. At the molecular level, cold stress triggers an intricate transcriptional regulatory network. Activated transcription factors like MYB, WRKY, bHLH, and bZIP bind to the promoter regions of stress-responsive genes. These genes can be broadly classified as either Early Cold-responsive Genes (EBGs) or Late Cold-responsive Genes (LBGs) (Fig. 8) [86]. EBGs are rapidly generated and involved in signal transduction and transcriptional control, whereas LBGs support long-term stress adaptation. One of the primary cold-signalling mechanisms identified is the CBF–COR (C-repeat binding factor–cold-responsive) pathway. Under cold stress, CBF transcription factors activate COR genes, which encode proteins involved in osmoprotection, membrane integrity, and antioxidant activity. To increase cold tolerance, this pathway is crucial. One important consequence of these transcriptional changes is the accumulation of flavonoids, an important class of secondary metabolites [86]. Flavonoids are strong non-enzymatic antioxidants that assist enzymatic defenses and directly scavenge Reactive Oxygen Species (ROS). They also help maintain membranes under cold stress and modulate signals. The diagram links secondary metabolism to stress signalling by illustrating how a number of transcription factors affect flavonoid synthesis through EBGs and LBGs. All things considered, the figure provides comprehensive knowledge of how plants coordinate changes at the membrane, metabolic, and gene expression levels in response to cold stress. By enhancing membrane integrity, regulating ROS through antioxidant systems, triggering stress-related transcription factors, and activating flavonoids, plants effectively reduce cold-induced damage and promote survival under low-temperature conditions [86].
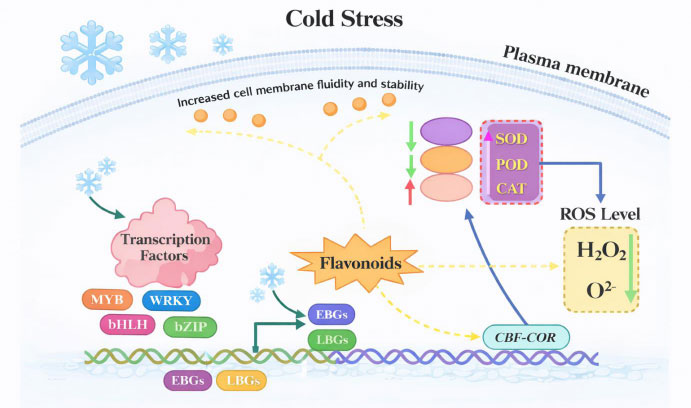
Mechanism of flavonoids under cold stress.
3.7.3. Role of Phenolic Compounds
Abiotic stress will affect the levels of different phenolics (Table 19), which act as stress signals, photoprotectants, and ROS scavengers under stressful conditions (Table 18). The most potent antioxidants and free-radical scavengers are stilbenes. One fundamental aspect of lignans' beneficial effect in plant abiotic stress responses and tolerance is their antioxidant activity. When it comes to a plant's reaction to harmful heavy metals, flavanols are important mediators. It has been suggested that isoflavone accumulation is a sign of salt tolerance. Compared to monohydroxy flavones, quercetin and dihydroxyflavones are better at dispersing damaging UV-B light [87].
| Phenolic Compounds | Uses |
|---|---|
| Anthocyanins | ROS scavengers |
| Stilbenes | Strongest antioxidant and free-radical scavenging |
| lignans | Antioxidant activity |
| Isoflavone | Marker of salt tolerance (accumulation) |
3.8. Nitrogen-containing Compounds
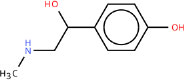
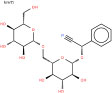
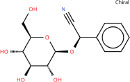
Common amino acids are used in the biosynthesis of nitrogenous secondary metabolites. They include cyanogenic glycosides, which are of great interest due to their therapeutic qualities and human toxicity [49].
Alkaloids and cyanogenic glycosides are highlighted in Fig. (9), which depicts nitrogen-based plant defenses. While cyanogenic glycosides produce poisonous molecules following tissue damage, alkaloids play pharmacological and defensive roles against herbivores and pathogens, forming an efficient chemical defense system that improves plant survival under biotic stress. Classification and sources of nitrogen-containing compounds are presented in Table 20.
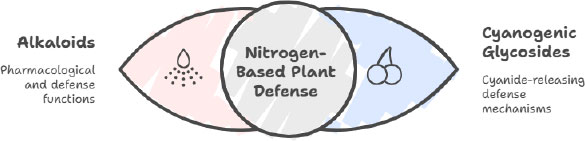
Classification of nitrogen-containing compounds.
3.8.1. Alkaloids
In these compounds, the nitrogen atom is typically a component of a heterocyclic ring, which is made up of both carbon and nitrogen atoms. The most notable pharmacological effects of alkaloids on vertebrate animals are well-known. Typically, alkaloids are produced from one of a few common amino acids, specifically tryptophan, tyrosine, and lysine.
3.8.2. Cyanogenic Glucosides
When the plant is crushed, two families of these substances, cyanogenic glycosides and glucosinolates, are readily broken down, releasing volatile toxic compounds. However, the parent compounds themselves are not toxic. The well-known toxic gas Hydrogen Cyanide (HCN) is released by cyanogenic glycosides.
CONCLUSION
Abiotic stresses, including drought, salinity, temperature extremes, high light intensity, and nutrient imbalance, significantly influence plant growth, fruit yield, and the biosynthesis of bioactive compounds in fruit crops. Evidence summarized in this review indicates that moderate drought stress enhances the accumulation of phenolic compounds and flavonoids in crops such as grape, strawberry, and pomegranate, while salinity promotes the synthesis of phenolics, carotenoids, and antioxidant compounds in tomato and other salt-tolerant fruit species. Likewise, low-temperature stress stimulates anthocyanin accumulation in fruits such as grape and blueberry, whereas high light intensity enhances flavonoid and carotenoid biosynthesis in several fruit crops. Although severe stress conditions generally reduce fruit productivity and quality, controlled or moderate stress can activate antioxidant defence mechanisms and secondary metabolic pathways, leading to improved nutritional and functional quality of fruits.
Overall, this review demonstrates that the response of bioactive metabolites to abiotic stress is both crop- and stress-specific, with phenolics, flavonoids, anthocyanins, carotenoids, and other antioxidants showing distinct patterns of accumulation depending on the type and intensity of stress. These stress-induced metabolic changes not only improve the antioxidant potential and health-promoting properties of fruits but also provide opportunities for developing sustainable crop management strategies and breeding programmes aimed at producing climate-resilient fruit cultivars with enhanced nutritional quality. Future research should focus on optimizing stress management practices and elucidating the molecular mechanisms regulating metabolite biosynthesis across different fruit species to maximize both yield stability and fruit quality under changing climatic conditions.
AUTHORS’ CONTRIBUTIONS
The authors confirm their contribution to the paper as follows: G.K.: Study conception and design; U.C and A.O.: Data collection; U.C. and A.O.: Writing –original draft preparation; M. and J.D.: Writing –review and editing; B.A. and G.R.S.: Draft manuscript. All authors reviewed the results and approved the final version of the manuscript.
LIST OF ABBREVIATIONS
| ROS | = Reactive Oxygen Species |
| HPLC | = High-Performance Liquid Chromatography |
| GDD | = Growing Degree Days |
| UV | = Ultraviolet radiation |
| GC-MS | = Gas Chromatography Mass Spectroscopy |
| CH | = Chilling Hours |
ACKNOWLEDGEMENTS
Declared none.