All published articles of this journal are available on ScienceDirect.
Advances in Wheat (Triticum aestivum L.) Genetics, Genomics and Breeding: Current Status, Tools and Future Perspectives for Sustainable Food Security
 iD
Mankesh Kumar1
iD
Chandan Kishore1
iD
Authors Info & Affiliations
Abstract
Wheat (Triticum aestivum L.) is one of the most important cereal crops in the world. It supplies nearly 18–20% of global dietary calories and protein, sustaining the food security of over 2.5 billion people. Global food demand is projected to increase by 35–56% by 2050, placing additional pressure on wheat production and improvement programmes and making genetic improvement an urgent priority. This review synthesizes current advances in wheat genetics, genomics, and breeding. It discusses the origin and domestication of wheat, as well as the structure of the allohexaploid genome (AABBDD; 2n = 6x = 42). Major genes and Quantitative Trait Loci (QTLs) governing yield, disease resistance, grain quality, and abiotic stress tolerance are critically reviewed. Key breeding approaches are evaluated, including doubled haploid technology, Marker-Assisted Selection (MAS), Genomic Selection (GS), speed breeding, and CRISPR/Cas9 genome editing. Stability analysis methods, particularly the Additive Main Effects and Multiplicative Interaction (AMMI) model and the Eberhart–Russell regression, are discussed in the context of multi-environment trial evaluation. The integration of Genome-Wide Association Studies (GWAS), pangenomics, multi-omics, and high-throughput phenotyping for precision wheat improvement is also covered. This review focuses primarily on India, with special attention to the North Eastern Plains Zone (NEPZ) and the eastern Indo-Gangetic Plains. In this region, terminal heat stress and monsoon variability pose major production challenges. Key challenges and strategic recommendations for developing climate-resilient, high-yielding, and nutritionally superior wheat varieties are outlined.
1. INTRODUCTION
Wheat (Triticum aestivum L.) is one of the most important food crops globally and the most widely cultivated cereal by area. It is cultivated on approximately 220 million hectares and produces over 780 million tonnes of grain annually [1]. It provides nearly one-fifth of the total calories and protein consumed worldwide. It is particularly central to food and nutritional security across South Asia, Central Asia, North Africa, and Europe [2]. In India, wheat is the second most important staple crop, with production of approximately 110.6 million tonnes in 2022–23. For the purpose of varietal development and recommendation, India is divided into six agro-climatically distinct wheat-growing zones (Zone I to Zone VI), each characterized by unique soil, temperature, and rainfall conditions. Bihar, located in the eastern Indo-Gangetic Plains (EIGP), falls under Zone III, i.e., the North Eastern Plains Zone (NEPZ), which covers eastern Uttar Pradesh, Bihar, Jharkhand, Odisha, West Bengal, Assam, and the plains of north-eastern states. This zone is recognized for its unique cropping conditions including late sowing, terminal heat stress, and high humidity, making productivity enhancement a major national priority.
Global food demand is projected to increase by 35–56% by 2050 owing to rapid population growth, rising incomes, and shifting dietary patterns, placing additional pressure on wheat production and improvement programmes [3]. However, the annual rate of genetic gain in wheat yield has declined to approximately 0.9–1.1% per year in major producing countries, falling short of the 1.7% annual increase required [4, 5]. Some recent Indian estimates place the required rate even higher, at 2.4% per year [6]. Simultaneously, climate change is intensifying the frequency and severity of abiotic stresses such as terminal heat, drought, and erratic rainfall, which disproportionately impact wheat productivity in the EIGP region [7, 8]. The emergence of highly virulent pathogen races, including Ug99 stem rust [9] and new yellow rust biotypes, further threatens yield stability.
The completion of the reference genome sequence for bread wheat by the International Wheat Genome Sequencing Consortium [10] and subsequent pangenome assemblies [11] have transformed the genomics landscape for wheat research. These resources, integrated with advanced genotyping platforms, high-throughput phenotyping, and multi-omics analytical methods, are being leveraged to accelerate the discovery of genes and QTLs governing complex agronomic traits. Modern breeding technologies, including genomic selection, speed breeding, and CRISPR-based genome editing, are shortening the breeding cycle and enabling more precise manipulation of the wheat genome [12, 13].
Stability analysis is an indispensable component of multi-environment evaluation of wheat genotypes. Given the vast diversity of agro-climatic environments across India and the rest of the world, identifying genotypes that yield consistently across locations is a key breeding objective. Statistical models such as the Eberhart–Russell [14] regression model and AMMI [15] model provide powerful frameworks for partitioning Genotype × Environment Interaction (GEI) and selecting broadly adapted or specifically adapted genotypes. The present review integrates multiple dimensions of wheat improvement research and identifies priority areas for future research and investment.
2. ORIGIN, DOMESTICATION AND EVOLUTIONARY HISTORY
Wheat is one of the first crops domesticated by humanity, with origins tracing back approximately 10,000–12,000 years to the Fertile Crescent of the Near East [16]. The domestication of wheat from wild progenitors involved the selection of key traits including non-brittle rachis (preventing grain shattering), free-threshing grains, an erect growth habit, and a modified photoperiod response. These traits are collectively termed the ‘domestication syndrome’ [17]. Bread wheat (T. aestivum, 2n = 6x = 42; AABBDD) arose through two sequential polyploidization events. The first involved hybridization between Triticum urartu (A genome) and a species related to Aegilops speltoides (B genome). This produced tetraploid emmer wheat (T. dicoccoides, AABB; 2n = 4x = 28) approximately one million years ago. Subsequently, ~8,000–9,000 years ago, cultivated emmer hybridized with Aegilops tauschii (D genome donor) to give rise to hexaploid bread wheat [18]. The complete evolutionary pathway is presented in Fig. (1). Key domestication genes include the Q gene governing the free-threshing habit, Br (brittle rachis loci), and the vernalization and photoperiod response genes (Vrn and Ppd). Modern cultivars retain only a fraction of the genetic diversity present in wild progenitors and landraces due to repeated bottlenecks during domestication and subsequent breeding [19, 20]. This underscores the importance of exploiting wild relatives and landraces as sources of novel alleles for contemporary wheat improvement.
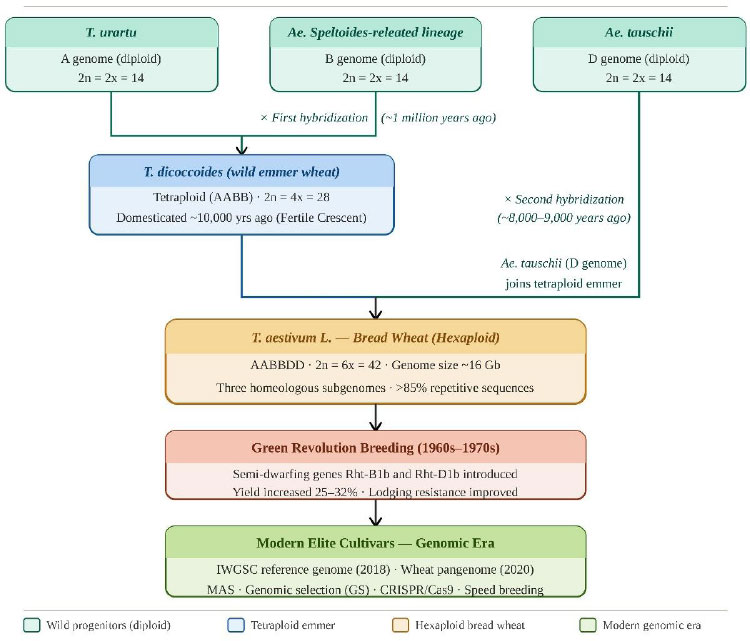
Evolutionary pathway of wheat from wild diploid progenitors to modern bread wheat (Triticum aestivum L.; AABBDD; 2n = 6x = 42) through two sequential allopolyploidisation events, showing key milestones of the Green Revolution and the genomic era (Image adapted from subsequent studies [17, 18]).
Abbreviations: CRISPR = clustered regularly interspaced short palindromic repeats; IWGSC = International Wheat Genome Sequencing Consortium; MAS = marker-assisted selection; Rht = Reduced height.
3. GENOME STRUCTURE, ORGANIZATION AND GENETIC DIVERSITY
3.1. Genome Structure and Complexity
The bread wheat genome is one of the largest and most complex among cultivated plants. It has an estimated size of approximately 16 Gb, distributed across 21 chromosome pairs and organized into three homeologous subgenomes (A, B, D) [10]. More than 85% of the genome consists of repetitive sequences, primarily transposable elements; this complicates genome assembly, gene annotation, and functional analysis. The IWGSC reference genome assembly (cultivar Chinese Spring) annotated approximately 107,891 high-confidence protein-coding genes, providing an unprecedented resource for wheat genomics and breeding research [10]. Multiple chromosome-level assemblies of diverse accessions have since been generated, forming the foundation for pangenome analysis.
3.2. Pangenomics and Haplotype Diversity
The wheat pangenome is assembled from the genomes of multiple diverse accessions. It captures the full range of gene content within the species, including core genes (present in all accessions) and dispensable genes (present in only some accessions). A 10-genome pangenome assembly identified approximately 140,500 protein-coding gene loci, of which approximately 22% were Presence-Absence Variants (PAVs) [11]. These PAVs are frequently associated with environmental adaptation, disease resistance, and variation in grain quality. Haplotype analysis of PAV regions has become a powerful approach for identifying novel alleles across global germplasm collections. The development of pangenome resources has substantially expanded the tractable genetic diversity for wheat improvement beyond what is accessible through single reference genome analysis. More recently, long-read sequencing technologies (PacBio HiFi and Oxford Nanopore) have enabled the assembly of chromosome-scale, near-complete genomes of diverse wheat accessions. This has substantially advanced the resolution and completeness of haplotype-based pangenome analyses beyond the initial 10-genome reference [21]. In 2025, a telomere-to-telomere assembly of hexaploid bread wheat was completed, providing a near-complete, highly contiguous view of the wheat genome from end to end [22]. These high-quality assemblies are revealing structural variation, complex repeats, and novel gene families that were inaccessible through short-read sequencing, accelerating both gene discovery and deployment of pangenome-based breeding strategies. Recent syntheses have situated wheat-specific advances within the broader trajectory of crop pangenomics, underscoring its growing role in trait dissection, biodiversity conservation, and breeding decision-making across species [23, 24]. Illustrating this momentum, a 17-genome pangenome of Chinese wheat cultivars has resolved structural variants linked to breeding history, vernalization habit, and local adaptation, providing direct empirical support for haplotype-informed selection strategies [25].
3.3. Genetic Diversity and Germplasm Resources
Despite the complexity of its genome, modern elite wheat germplasm has a relatively narrow genetic base. SNP array and whole-genome resequencing studies have demonstrated that elite cultivars share approximately 90–95% of genomic content, reflecting the repeated use of a small number of elite parents in breeding programmes [20]. A comprehensive diversity analysis of over 80,000 wheat accessions using the DArTseq platform recently revealed distinct selection footprints in modern germplasm and highlighted under-utilized genetic material as a valuable resource for pre-breeding [26]. This genetic bottleneck severely limits the availability of novel alleles for future improvement. Major germplasm repositories including CIMMYT (Mexico), ICARDA (Lebanon/Morocco), NBPGR (New Delhi), and USDA-GRIN collectively conserve over 800,000 wheat accessions. Wild relatives of wheat, particularly Aegilops species, Agropyron, and Thinopyrum, are recognized reservoirs of novel alleles for disease resistance, drought tolerance, heat tolerance, and nutritional quality [27, 28]. For disease resistance specifically, wild relatives from both primary and secondary gene pools have been shown to continue providing valuable and unique resistance alleles not present in cultivated hexaploid wheat [28]. This finding underscores their strategic importance for durable resistance breeding. Synthetic hexaploid wheat lines, produced by hybridizing tetraploid wheat with Ae. tauschii, have been a major strategy for introducing D-genome diversity into elite germplasm [29].
4. MAJOR GENES AND QTLs FOR ECONOMICALLY IMPORTANT TRAITS
A summary of major genes and QTLs governing key agronomic traits in wheat is presented in Table 1.
| Trait Category | Gene / QTL | Chromosome | Effect / Function | Key Reference |
|---|---|---|---|---|
| Yield/Dwarfism | Rht-B1b, Rht-D1b | 4B, 4D | Semi-dwarfism; improved harvest index; lodging resistance | [30] |
| Yield/Grain Weight | TaGW2-A1 | 6AS | Natural expression variation and a characterized G2373A splice-acceptor loss-of-function allele are associated with increased grain weight and grain dimensions | [31] |
| Leaf Rust (APR) | Lr34, Lr46, Lr67, Lr68 | 7D, 1B, 4D, 7B | Durable adult plant resistance; partial, broad-spectrum; Lr34=Sr57/Yr18 (pleiotropic) | [9, 32] |
| Leaf Rust (Race-specific) | Lr37 (T2NS.2AS) | 2A | Race-specific; from Ae. ventricosa; overcome by some virulent races; use with APR | [9, 33, 34] |
| Yellow Rust (APR) | Yr18 (=Lr34/Sr57), Yr46 (=Lr67/Sr55) | 7D, 4D | Durable APR; pleiotropic multi-pathogen resistance; slow-rusting | [9, 35] |
| Yellow Rust (Race-specific) | Yr5, Yr7, YrSP | 2BL, 2BL, 2BL | Race-specific (all-stage); Yr5, Yr7 and YrSP encode BED-domain NLRs; Yr5 remains broadly effective against prevailing Pst races, while Yr7 and YrSP have been overcome; Yr17 (T2NS translocation) has been overcome by new races. Yr15 virulence was detected in the United Kingdom in 2025, reported as the first large-scale breakdown of this gene recorded globally [36] | [9, 34, 36, 37] |
| Stem Rust (Race-specific) | Sr22, Sr25, Sr26, Sr33, Sr35, Sr45, Sr50 | 7A, 7D, 6A, 1D, 3A, 1D, 1D | Effective against Ug99; most valuable in combinations to delay breakdown | [9, 34] |
| Stem Rust (APR) | Sr2, Sr55(=Lr67), Sr57(=Lr34), Sr58(=Lr46) | 3BS, 4D, 7D, 1B | Non-race-specific APR; slow-rusting; multi-pathogen pleiotropic genes | [9, 35] |
| FHB Resistance | Fhb1 | 3BS | Type II FHB resistance; Sumai 3-derived | [38] |
| Powdery Mildew | Pm21, TaMLO | 6VS/6AL, 4A/4B/4D | Pm21: race-specific; TaMLO: susceptibility-gene family; TALEN-mediated mutation of all three homoeologs conferred heritable broad-spectrum powdery mildew resistance | [39, 40] |
| Breadmaking Quality | Glu-D1 (5+10 subunit) | 1D | Gluten protein composition associated with dough and breadmaking quality | [41] |
| Grain Protein/Micronutrients | Gpc-B1 (NAC-TF) | 6B | Increases grain protein, Zn and Fe; biofortification target | [42] |
| Heat Stress Tolerance | QTLs: 2B, 7B, 7D | Multiple | CTD, Grain Weight (TGW), and grain-filling duration under heat; reported QTLs require multi-environment validation in NEPZ germplasm | [43] |
| Drought Tolerance | TaDREB1, TaWRKY, TaMYB | Multiple | DREB/CBF pathway; osmotic adjustment; root architecture in wheat | [44, 45] |
| Salinity Tolerance | Nax1 (2AL); Nax2/TmHKT1;5-A (5A) | 2AL, 5A | Nax1: sodium exclusion in durum wheat [46]; Nax2/TmHKT1;5-A: xylem Na+ retrieval and reduced leaf Na+ accumulation [47] | [46, 47] |
| Photoperiod Response | Ppd-D1, Ppd-B1 | 2D, 2B | Photoperiod insensitivity; adaptation to diverse environments | [17] |
| Vernalization | Vrn-A1, Vrn-B1, Vrn-D1 | 5A, 5B, 5D | Spring vs. winter growth habit; flowering time | [17] |
4.1. Yield and Yield Components
Grain yield in wheat is a complex quantitative trait governed by numerous genes and QTLs distributed across the three subgenomes. The semi-dwarfing genes Rht-B1b and Rht-D1b were the cornerstone of the Green Revolution. By reducing plant height and lodging susceptibility and improving harvest index, they underpinned the substantial wheat yield gains of the Green Revolution in Asia and Europe during the 1960s and 1970s [30]. The gene TaGW2 (Grain Width and Weight 2) negatively regulates grain width and weight; reduced TaGW2 expression is associated with wider, heavier grains [31], and a loss-of-function splice acceptor site mutation in TaGW2-A1 increased thousand-grain weight by 6.6%, grain width by 2.8%, and grain length by 2.1% in tetraploid and hexaploid backgrounds [31]. Major QTLs for yield components have been mapped on chromosomes 4A, 4B, 4D, 6B, and 7D.
4.2. Disease Resistance Genes
More than 80 Leaf rust resistance (Lr) genes, over 90 Yellow rust resistance (Yr) genes, and more than 60 Stem rust resistance (Sr) genes have been catalogued in wheat, with continuous additions as wild relative germplasm is screened [9, 33]. Durable Adult Plant Resistance (APR) genes for leaf rust include Lr34, Lr46, Lr67, and Lr68. These loci generally confer partial, durable adult-plant resistance and are valuable components of resistance gene pyramids; their frequency and effectiveness should be assessed within the target breeding population and pathogen context [9, 32]. The gene Lr37 (from the T2NS.2AS translocation from Aegilops ventricosa) confers race-specific leaf rust resistance, but it has been overcome by some virulent Puccinia triticina races and should be deployed in combination with APR genes [9].
For yellow rust (Puccinia striiformis f. sp. tritici; Pst), key resistance genes in Indian breeding include the race-specific Yr10, Yr15, and Yr17, and the durable APR genes Yr18 (=Lr34/Sr57) and Yr46 (=Lr67/Sr55/Pm46) [9, 35]. In addition, the race-specific genes Yr5, Yr7 and YrSP, which map to chromosome arm 2BL and encode nucleotide-binding leucine-rich-repeat proteins carrying an integrated zinc-finger BED domain, confer all-stage resistance; Yr5 remains highly effective, with only two of more than 6,000 Pst isolates tested worldwide found virulent, whereas Yr7 and YrSP have been overcome in the field, so these genes should be deployed in gene pyramids and monitored through regional pathotype surveillance [37]. Notably, Yr17 (part of the Lr37/Sr38/Yr17 complex on the T2NS.2AS translocation from Ae. ventricosa) is no longer effective against new virulent Pst races. Sr38, carried on the same translocation, is similarly ineffective against Ug99 Pgt races. Deployment of these genes must therefore be supplemented by pyramiding with functional APR genes or additional race-specific genes [9].
The emergence of Ug99 stem rust race (TTKSK; the pathotype designation code) in East Africa and its subsequent virulent lineages have renewed interest in effective Sr genes. Race-specific resistance genes are individually effective against Ug99 derivatives but are most valuable when deployed in combinations to delay resistance breakdown. These genes include Sr22, Sr25, Sr26, Sr33, Sr35, Sr45, and Sr50 [9, 48]. Non-race-specific Adult Plant Resistance (APR) genes confer slow-rusting, partial resistance not readily overcome by individual virulent races. These genes include Sr2, Sr55 (=Lr67/Yr46/Pm46), Sr57 (=Lr34/Yr18/Pm38/Sb1/Ltn1), Sr58 (=Lr46/Yr29/Pm39), and Sr63. Their value in durable resistance programmes is well established [9, 35]. A landmark finding in durable rust management has been the identification of three pleiotropic APR genes: Sr55 (=Lr67/Yr46/Pm46), Sr57 (=Lr34/Yr18/Pm38/Sb1/Ltn1), and Sr58 (=Lr46/Yr29/Pm39) [33, 35]. Each of these three genes confers slow-rusting, partial, non-race-specific resistance simultaneously against stem rust, leaf rust, yellow rust, and powdery mildew, providing multi-pathogen protection from a single genetic locus. Collectively, such pleiotropic and adult-plant resistance genes are among the most valuable and durable components available to wheat breeding programmes, particularly when pyramided with race-specific resistance genes [9, 35]. The gene Sr57 (=Lr34/Yr18) is also located at the same locus as Sb1 (spot blotch resistance against Bipolaris sorokiniana) and Bdv1 (barley yellow dwarf virus tolerance), exemplifying the exceptional pleiotropic value of this gene for wheat breeding in humid environments [9]. The Fhb1 locus (chromosome 3BS), originally identified in Chinese wheat cv. Sumai 3, is a major source of Type II resistance and the most effective QTL for Fusarium Head Blight (FHB) resistance, and has been widely used in FHB-resistance breeding programmes [38, 49]. Powdery mildew resistance genes Pm21 (race-specific, from Haynaldia villosa via 6VS/6AL translocation) and TALEN-mediated mutation of all three TaMLO homoeologs (conferring heritable broad-spectrum mlo-mediated resistance) represent contrasting genetic strategies for powdery mildew management [39, 40].
4.3. Grain Quality Genes
Wheat grain quality is largely determined by gluten proteins, particularly High-Molecular-Weight Glutenin Subunits (HMW-GS) encoded by Glu-A1, Glu-B1, and Glu-D1 loci. The HMW-GS allele combination 5+10 at Glu-D1 has been associated with favourable dough rheological properties and breadmaking-quality traits, relative to the 2 + 12 allele in comparative studies [50]. Waxy (Wx) genes controlling amylose content are important for noodle and food processing quality. The Gpc-B1 locus on chromosome 6B, encoding a NAC transcription factor, regulates grain protein, zinc, and iron concentrations and is an important target for biofortification breeding [42, 51].
4.4. Abiotic Stress Tolerance
Terminal heat stress is one of the most serious threats to wheat production in the EIGP. Key QTLs for heat tolerance have been mapped on chromosomes 2B, 7B, and 7D, associated with canopy temperature depression, grain weight, and grain-filling rate under heat stress [43]. TaDREB/CBF and TaWRKY transcription factors have been implicated in abiotic-stress signalling in wheat and related experimental systems [44, 45]. The TaELF3 gene modulates photoperiod response and heat escape. The Nax1 locus was mapped to chromosome arm 2AL in durum wheat and accounted for approximately 38% of the phenotypic variation in leaf-blade Na+ concentration [46]. At the Nax2 locus, TmHKT1;5-A contributes to reduced Na+ transport to leaves through xylem Na+ retrieval [47].
5. WHEAT BREEDING STRATEGIES: CLASSICAL AND MODERN APPROACHES
A comparative overview of major wheat breeding strategies is presented in Table 2. The integrated modern wheat breeding pipeline is illustrated in Fig. (2).
| Method | Key Advantages | Limitations | Time to Variety | Example Applications |
|---|---|---|---|---|
| Conventional Hybridization | No special technology; proven track record | Slow; phenotypic selection confounded by GEI | ~12 years | Pedigree, bulk, backcross methods; AICRP wheat trials [52, 53] |
| Doubled Haploid (DH) | Instant homozygosity; saves 6–8 inbreeding generations | Genotype-dependent tissue culture; albinism | ~6–7 years | Mapping populations; elite line fixation in CIMMYT [54] |
| Marker-Assisted Selection (MAS) | Early-generation seedling selection; precise major gene transfer | Effective mainly for major-gene loci; linkage drag | ~8–10 years | Lr34, Sr31, Fhb1, Pm21, Glu-D1 introgression programmes [55] |
| Genomic Selection (GS) | Improves polygenic traits; shortens cycle; higher gain per year | Requires large training set and genotyping costs | ~4–6 years | CIMMYT international nurseries; yield and quality GS [56, 57] |
| Speed Breeding | 6 generations per year; compatible with MAS and GS | Controlled environment; high infrastructure cost | Accelerates generation advancement (up to ~6 generations/year in suitable spring wheat); end-to-end cultivar release still depends on crossing design, field evaluation, seed multiplication, and national release requirements | CIMMYT, Univ. Queensland, Rothamsted Research [12, 58] |
| CRISPR/Cas9 Editing | Precise multiplex editing across homeologs; novel variation | Regulatory hurdles; transformation efficiency limits broad adoption | Variable | TaMLO (mildew), TaGW2 (grain weight), TaDEP1 (yield) [40, 59, 60] |
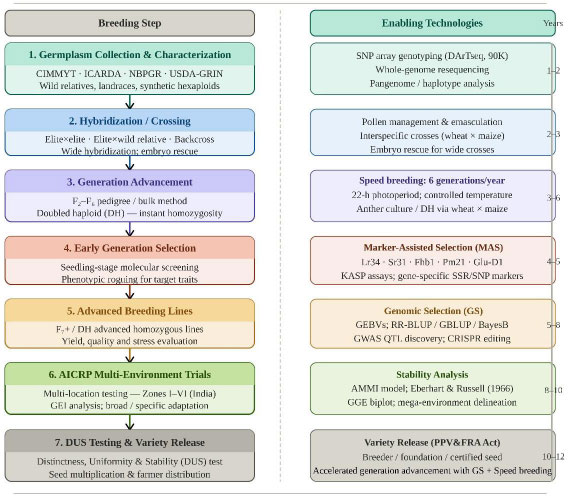
Integrated wheat breeding pipeline from germplasm collection to variety release, with enabling biotechnological tools and approximate cumulative timeline. (Image adapted from previous studies [12, 13]).
Abbreviations: AICRP = All India Coordinated Research Project; AMMI = Additive Main effects and Multiplicative Interaction; CIMMYT = International Maize and Wheat Improvement Center; CRISPR = clustered regularly interspaced short palindromic repeats; GEBVs = genomic estimated breeding values; GEI = genotype × environment interaction; GBLUP = genomic best linear unbiased prediction; GGE = genotype main effect plus genotype-by-environment interaction; GWAS = genome-wide association study; ICARDA = International Center for Agricultural Research in the Dry Areas; KASP = kompetitive allele-specific PCR; NBPGR = National Bureau of Plant Genetic Resources; PPV&FRA = Protection of Plant Varieties and Farmers’ Rights Authority; QTL = quantitative trait locus; RR-BLUP = ridge-regression best linear unbiased prediction; SNP = single nucleotide polymorphism; SSR = simple sequence repeat; USDA-GRIN = United States Department of Agriculture Germplasm Resources Information Network.
5.1. Conventional Breeding
Conventional wheat breeding based on hybridization and selection continues to underpin national wheat improvement programmes in India and worldwide. The pedigree method, bulk population method, backcross method, and recurrent selection are the most widely used approaches. In India, the Indian Agricultural Research Institute (IARI), the ICAR-Indian Institute of Wheat and Barley Research (ICAR-IIWBR) Karnal, and Punjab Agricultural University (PAU) Ludhiana have made significant contributions. Despite its proven efficacy, conventional breeding is time-intensive, typically requiring 10–12 years from a cross to variety release, and relies on phenotypic selection that may be confounded by Genotype × Environment Interaction (GEI).
5.2. Doubled Haploid Technology
Doubled Haploid (DH) technology produces completely homozygous lines in a single generation through anther culture or wheat × maize wide hybridization, bypassing the 6–8 generations required for inbreeding in conventional programmes. DH lines have been widely used in wheat for developing mapping populations and accelerating elite line development [54]. Limitations include genotype-dependent tissue-culture responses and albinism in some anther-derived plants, which constrain broad adoption across diverse genetic backgrounds.
5.3. Marker-assisted Selection
Marker-Assisted Selection (MAS) enables breeders to select desirable alleles at the seedling stage, reducing the influence of environmental variation and accelerating the breeding cycle. The evolution from RFLPs and SSRs to high-density SNP arrays has substantially expanded the capacity of MAS. It has been particularly effective for introgression of major gene loci such as Lr34, Sr31, Pm21 (powdery mildew resistance), Fhb1 (FHB resistance), and Glu-D1 (breadmaking quality) into elite backgrounds [55]. Institutions including IARI New Delhi have applied MAS in developing rust-resistant and FHB-resistant varieties for the Indian subcontinent.
5.4. Genomic Selection
Genomic Selection (GS) is a genome-wide prediction approach that uses dense marker data to estimate Genomic Estimated Breeding Values (GEBVs) for all candidates in a population. This approach enables selection of complex quantitative traits without prior identification of specific QTLs [56]. Statistical models including RR-BLUP, GBLUP, BayesB (a Bayesian variable-selection genomic model), and machine learning methods have been applied to wheat GS [13, 61]. Genomic selection can shorten breeding cycles and increase genetic gain per unit time when robust, routinely updated training populations and high-quality phenotypes are available; the magnitude of benefit is programme-, trait-, and environment-specific and should be empirically evaluated within each breeding pipeline [62]. CIMMYT semi-arid wheat trials have reported realised genetic gains of approximately 1.4–1.8% per year, with the highest relative rate recorded in low-yielding environments [63]. These gains reflect the performance of the combined breeding system and should not be attributed solely to genomic selection.
5.5. Speed Breeding
Speed breeding accelerates plant generation advancement by extending the photoperiod to 22 hours and manipulating temperature in controlled growth facilities. Under speed-breeding conditions, spring wheat can complete up to six generations per year, compared with 1–2 field generations [12]. Speed breeding, when integrated with genomic selection and marker-assisted selection, substantially compresses the breeding cycle and is now adopted in major programmes at CIMMYT, the University of Queensland, and Rothamsted Research [58]. Combining speed breeding with genomic selection can increase genetic gain per unit time by shortening generation intervals and improving selection efficiency [13, 64, 65]. Wider adoption still faces practical barriers. These include the cost of controlled-environment facilities, limited technical training, and the need for reliable electricity and cooling infrastructure, which are especially relevant for SAUs in the NEPZ [64].
5.6. Genome Editing and CRISPR/Cas9
CRISPR/Cas9 enables targeted modification of specific genomic sequences, including simultaneous editing of all three homeologous gene copies in hexaploid wheat. Multiplex mutation of TaMLO homoeologs conferring heritable powdery mildew resistance was first demonstrated using TALENs; the same study also demonstrated CRISPR/Cas9 editing of TaMLO-A1 [40]. Subsequent reports include editing of TaGW2 for increased grain weight, TaGASR7 for grain weight improvement using DNA-free RNP delivery, and TaDEP1 for enhanced spike architecture [59, 66]. The development of GRF4–GIF1 chimeric gene approaches has significantly improved wheat transformation efficiency, broadening the applicability of CRISPR across diverse elite genotypes [67]. Base editing and prime editing platforms are being adapted for wheat to allow precise single-nucleotide changes without double-strand breaks. Complementary approaches using transgenic overexpression of wheat transcription factors (e.g., TaCR4-A) have also significantly improved grain size and weight [68]. Comprehensive reviews of CRISPR/Cas applications in crop improvement underscore the transformative potential of precision genome editing for wheat breeding [60].
5.7. Critical Appraisal: A SWOT Analysis of Wheat Breeding Strategies for Indian Breeding Programmes
A critical review must move beyond description to evaluate breeding strategies against the practical constraints and opportunities of the target breeding system. Table 3 [12, 40, 55, 57] presents a structured SWOT (Strengths, Weaknesses, Opportunities, Threats) analysis of four key modern breeding strategies. These are Marker-Assisted Selection (MAS), Genomic Selection (GS), Speed Breeding, and CRISPR/Cas9 Genome Editing. These strategies are evaluated specifically in the context of Indian Council of Agricultural Research (ICAR) national institutes and State Agricultural Universities (SAUs) operating within the Indian wheat breeding infrastructure, with special consideration of the NEPZ (North Eastern Plains Zone).
| Strategy | Strengths | Weaknesses | Opportunities | Threats |
|---|---|---|---|---|
| Marker-Assisted Selection (MAS) | Precise introgression of major genes (Lr34, Fhb1, Pm21); early-generation seedling selection; established KASP/SSR marker systems at IARI, ICAR-IIWBR, PAU; reduces GEI effect on selection. | Limited effectiveness for polygenic traits (yield, heat tolerance); linkage drag; requires prior QTL knowledge; Requires access to reliable marker platforms, validated assays, and technical capacity. | Declining KASP cost; integration with speed breeding for rapid gene pyramiding; ICAR BIG programme expanding MAS to SAUs; AICRP nurseries providing pre-selected advanced lines for SAU evaluation. | Rapid pathogen evolution overcoming pyramided resistance genes; over-reliance on narrow gene combinations; loss of effectiveness of Sr31 to Ug99 stem rust as precedent. |
| Genomic Selection (GS) | Superior for complex traits, including yield and heat tolerance; shortens cycle to 4–6 years; Can increase genetic gain per unit time when prediction accuracy, training-population relevance, and cycle time are optimized. | Requires large training population (>1,000 lines); requires sustained investment in genotyping, phenotyping, and data-analysis capacity; bioinformatics expertise needed; prediction accuracy declines across diverse environments; limited NEPZ-specific training data. | Declining genotyping costs (GBS platforms); NEPZ multi-environment data could support development of locally relevant training populations, subject to adequate phenotypic standardization and data governance; potential to build NEPZ-specific GS training populations. | GEI reduces prediction accuracy across zones; limited public funding for GS at most SAUs; technology gap between international centres and state universities; risk of genetic erosion under intense selection. |
| Speed Breeding | Up to 6 generations/year; compatible with MAS and GS in same generation; accelerates backcross conversion; scalable; eliminates seasonal constraints on generation advancement. | High infrastructure cost (growth chambers, LED lighting, climate control); not accessible at most Indian SAUs; photoperiod manipulation unsuitable for vernalization-requiring types; requires stable power supply. | Government investment in controlled environment facilities; modular, low-cost speed breeding chambers; high-altitude summer nurseries (Shimla/Manali) as a partial alternative; CIMMYT-CSISA protocol adoption. | Erratic power supply in Bihar/EIGP region; high recurring energy cost; genotype-specific differential response; field adaptation cannot be fully captured in controlled environments. |
| CRISPR/Cas9 Genome Editing | Precise multiplex editing of all three homeologs; creates novel variation beyond natural allele pools; potential to generate edited products without stable foreign-DNA integration when appropriate transient or DNA-free delivery methods are used; rapid functional validation of candidate genes. | Regulatory requirements in India vary by genome-editing category. Plants developed through SDN-1 or SDN-2 and free of exogenous introduced DNA are exempt from Rules 7–11 of the Rules, 1989, subject to the applicable 2022 guidelines and standard operating procedures; products outside these exempt categories require assessment under the applicable regulatory framework; low transformation efficiency in elite Indian genotypes; delivery system challenges; off-target assessment and molecular characterisation required at a level appropriate to the edit, delivery method, and applicable regulatory framework; whole-genome sequencing may be valuable in selected cases. | India’s 2022 framework, under which SDN-1 and SDN-2 genome-edited plants free of exogenous introduced DNA are exempt from specified provisions of the 1989 Rules, subject to the applicable guidelines and SOPs; improving wheat transformation protocols (GRF4-GIF1); potential to stack heat tolerance with rust resistance; public-private partnerships for gene editing platforms. | Uncertain regulatory requirements and assessment pathways for SDN-3 edits; public perception barriers; IP restrictions on CRISPR patents; significant time lag from gene editing to field-ready variety. |
6. STABILITY ANALYSIS OF WHEAT GENOTYPES IN MULTI-ENVIRONMENT TRIALS
The conceptual framework for stability analysis is depicted in Fig. (3) [69].
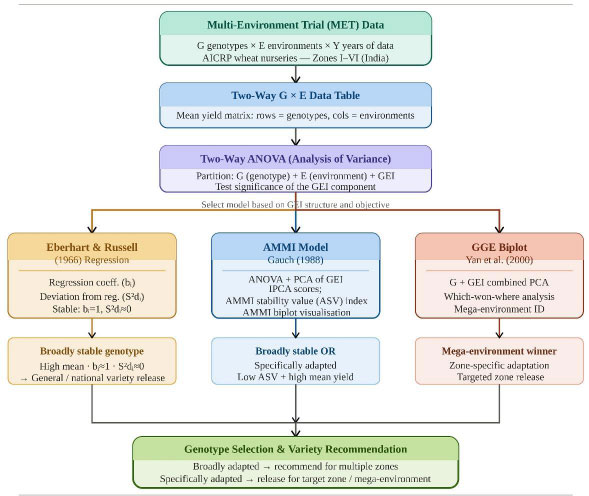
Analytical framework for stability analysis of multi-environment wheat trial data, illustrating pathways from G × E data assembly and two-way ANOVA to three alternative stability models converging on genotype selection and variety recommendation [14, 15, 69].
Abbreviations: AICRP = All India Coordinated Research Project; AMMI = Additive Main effects and Multiplicative Interaction; GEI = genotype × environment interaction; GGE = genotype main effect plus genotype-by-environment interaction; IPCA = interaction principal component axis; PCA = principal component analysis.
6.1. Genotype × Environment Interaction (GEI)
Genotype × Environment Interaction (GEI) occurs when genotypes differ in their relative performance across environments, complicating the selection of broadly adapted varieties. GEI is ubiquitous in wheat multi-location trials due to the wide diversity of soil types, temperature regimes, rainfall patterns, and crop management across the target environments of India. Effective partitioning and interpretation of GEI is essential for identifying stable, broadly adapted genotypes and for defining mega-environments for targeted varietal deployment [70].
6.2. Eberhart and Russell Regression Model
Eberhart and Russell [14] proposed a linear regression model that partitions the phenotypic response of a genotype across environments into: (i) the genotype mean (μi); (ii) the regression coefficient (bi, measuring response to improving environments); and (iii) the deviation from regression (S2di, measuring unpredictable stability). A broadly adapted, stable genotype is characterized by a mean yield above the trial mean, bi = 1 (average response to environmental change), and S2di ≈ 0 (consistent performance). Genotypes with bi > 1 are suited to high-input, favourable environments, while those with bi < 1 are adapted to low-input or stress environments. This model has been widely applied in AICRP wheat trials across India for variety evaluation [53].
6.3. AMMI Model
The AMMI (Additive Main effects and Multiplicative Interaction) model [15] combines ANOVA for additive main effects with Principal Component Analysis (PCA) for the multiplicative interaction component (GEI). The GEI sum of squares is decomposed into several Interaction Principal Component Axes (IPCAs), with each axis capturing a decreasing proportion of the GEI pattern. The AMMI Stability Value (ASV), calculated from the first two IPCA scores [71], provides a single numeric index for genotype stability: genotypes with low ASV are broadly stable, while a high ASV only reflects strong genotype × environment interaction; such genotypes can only be considered specifically adapted when the high ASV is paired with high mean performance in the target environment. The AMMI biplot, plotting IPCA1 against mean yield, allows simultaneous visualization of genotype mean performance and stability, facilitating identification of ideal genotypes [72].
6.4. GGE Biplot and Complementary Methods
The GGE biplot [69] combines Genotype (G) main effects with GEI into a single biplot, enabling ‘which-won-where’ pattern analysis, mega-environment delineation, and assessment of discriminating ability of test environments. Complementary stability statistics including Wricke’s ecovalence, Shukla’s stability variance, and Finlay–Wilkinson regression provide additional perspectives on GEI. A comparative summary of these stability analysis models is presented in Table 4. The selection of the most appropriate model depends on the structure and magnitude of GEI, as well as the specific objectives of the breeding programme.
Table 4.
| Feature | Eberhart and Russell [14] | AMMI Model [15] | GGE Biplot [69] | Finlay-wilkinson Regression |
|---|---|---|---|---|
| Statistical basis | Linear regression of genotype on environmental index | ANOVA + PCA of GEI | PCA of G + GEI | Linear regression on environment mean |
| Stability parameter | Regression coeff. (bi) and deviation (S2di) | AMMI Stability Value (ASV); IPCA scores | PC1 and PC2 scores; biplot | Regression coefficient (b) |
| Visual output | Scatter plot (bi vs. mean) | AMMI biplot (IPCA1 vs. IPCA2 or mean) | GGE biplot (PC1 vs. PC2) | Regression lines per genotype |
| GEI partitioning | Single regression captures linear GEI only | Multiple axes capture complex GEI patterns | G + GEI combined in single analysis | Linear component of GEI only |
| Mega-environment identification | Not directly applicable | Partially applicable via biplot clusters | Directly applicable (which-won-where) | Not applicable |
| Broadly stable genotype selection | bi = 1; S2di = 0; high mean yield | Low ASV; IPCA scores near origin; high mean | Close to the “ideal genotype” on the average-environment axis; high mean yield | b = 1; high mean yield |
| Key advantage | Simple; widely used; interpretable | Best GEI partitioning; flexible; graphical | Comprehensive visual analysis; mega-environment delineation | Simple; easy computation |
| Limitation | Assumes linear GEI only; less powerful for complex GEI | Computationally intensive; axis selection subjective | Intentionally combines G and GEI effects, so their individual contributions cannot be separated | Single regression may underfit complex GEI |
| Software | SPSS, SAS, R (agricolae) | R (agricolae, metan), GenStat | R (GGEbiplot), GenStat, Minitab | GenStat, SAS, R |
7. ADVANCED GENOMIC AND BIOTECHNOLOGICAL TOOLS
The multi-omics integration framework for wheat trait improvement is illustrated in Fig. (4) [73].
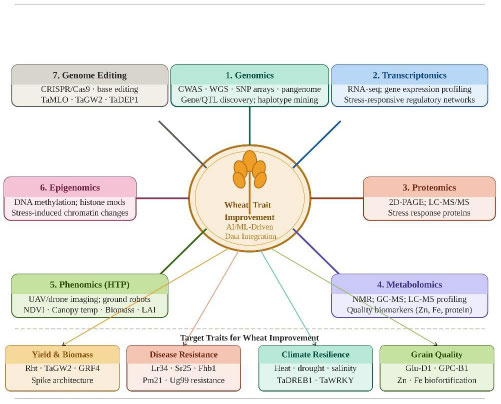
Integration of multi-omics and genomic tools for wheat trait improvement. Genomics, transcriptomics, proteomics, metabolomics, phenomics, GWAS, epigenomics, bioinformatics, and genome editing collectively inform wheat trait improvement and contribute to the development of climate-resilient, high-yielding, disease-resistant, and quality-enhanced wheat varieties (Image adapted from a previous study [73]).
Abbreviations: GWAS = genome-wide association study; QTL = quantitative trait locus; SNP = single nucleotide polymorphism; CRISPR = clustered regularly interspaced short palindromic repeats; GS = genomic selection; MAS = marker-assisted selection; NGS = next-generation sequencing.
7.1. Genome-wide Association Studies (GWAS)
GWAS leverages natural variation across diverse association panels to identify marker-trait associations at high mapping resolution, without the need to first develop a dedicated QTL mapping population. High-density SNP arrays (90K iSelect, 660K Axiom) and Genotyping-by-Sequencing (GBS) have enabled GWAS in large and diverse panels. Notable GWAS findings in wheat include associations for FHB resistance [74] and grain zinc and iron concentrations relevant to biofortification [75, 76]. GWAS results complement biparental QTL mapping by operating across a broader spectrum of haplotypic diversity.
7.2. High-throughput Phenotyping
High-Throughput Phenotyping (HTP) platforms include Unmanned Aerial Vehicles (UAVs) equipped with multispectral, thermal, and RGB cameras, ground-based robots, and controlled-environment imaging systems. These platforms have substantially expanded the capacity for precise, non-destructive phenotyping of large breeding populations. Key measurable traits include canopy temperature, Normalized Difference Vegetation Index (NDVI), leaf area index, biomass estimation, heading date, plant height, and lodging score. Integration of HTP data with genomic prediction models has been shown to improve accuracy for complex traits such as grain yield and drought tolerance [77-79].
7.3. Multi-omics Integration
Integration of genomics, transcriptomics, proteomics, metabolomics, and epigenomics (multi-omics) provides a holistic systems-level approach to deciphering the molecular mechanisms underlying complex agronomic traits in wheat. Transcriptomic analyses have identified key gene regulatory networks governing grain filling, response to terminal heat stress, and pathogen defence. Metabolomic profiling enables the identification of biomarkers for grain quality and stress tolerance. Epigenomic studies have revealed the role of DNA methylation and histone modifications in regulating gene expression under environmental stress. Artificial Intelligence (AI) and Machine Learning (ML) methods are increasingly applied to integrate multi-omics layers with phenotypic data to prioritize candidate genes and optimize selection decisions [73, 79]. In particular, multivariate deep learning architectures are being applied to integrate whole-genome marker data, hyperspectral imagery, and environmental covariates for genomic prediction of complex traits in wheat. These architectures include Convolutional Neural Networks (CNNs) and Long Short-Term Memory (LSTM) networks. These approaches have improved prediction accuracy in some wheat datasets, particularly when genomic, phenomic, and environmental covariates are integrated; however, performance relative to GBLUP and other conventional models is data- and validation-design-dependent, and independent evaluation is required before routine deployment [73, 79]. These deep learning frameworks represent a frontier of methodological development with potential relevance to the NEPZ wheat breeding context, though their application will require validation against NEPZ-specific training data. In this setting, multi-environment genomic prediction accuracy for terminal heat stress adaptation traits could be substantially improved by harnessing the non-linear relationships between marker profiles and environmental responses. This trajectory is corroborated by recent benchmarking studies in wheat genomic prediction and phenomic–genomic integration [80-82].
8. CHALLENGES AND FUTURE PERSPECTIVES
8.1. Key Challenges
Despite remarkable advances, several formidable challenges limit the pace of wheat genetic improvement. The narrow genetic base of elite germplasm, a product of progressive selection and genetic drift during domestication and breeding, restricts the availability of novel alleles for yield enhancement and stress adaptation. Climate change is steadily shifting temperature and rainfall regimes in major wheat-growing regions, making existing varieties increasingly less suited to emerging conditions [7, 83]. Rapidly evolving pathogen races, including new Ug99 lineages and virulent yellow rust strains, can overcome deployed resistance genes [9, 48, 84]. As described in Section 4.2, the emergence of Pst races virulent to widely deployed race-specific genes such as Yr17 [84] underscores the need for continued regional surveillance and resistance-gene monitoring. The continued emergence of virulent Pst biotypes, including those overcoming previously effective race-specific resistance genes, underscores the urgency of pyramiding multiple APR genes (Yr18, Yr46) and race-specific genes in new varieties. An additional emerging transboundary threat is wheat blast (Magnaporthe oryzae pathotype Triticum), which caused severe epidemics in eight southwestern districts of Bangladesh in 2016 with yield losses reaching up to 100% in affected fields under conducive conditions; the Bangladesh outbreak raised concern that wheat blast could spread to major wheat-producing areas in neighbouring South Asian countries; active surveillance and resistance-breeding preparedness are therefore warranted in the region [85]. The complex regulatory environment for gene-edited crops in India delays the translation of CRISPR-based innovations into field-ready varieties. Furthermore, the high cost of genotyping and phenotyping infrastructure remains a barrier to the adoption of genomic breeding in resource-limited national programme settings.
8.1.1. NEPZ-specific Challenges and Documented Breeding Outcomes
The North Eastern Plains Zone (NEPZ/Zone III), encompassing Bihar, eastern Uttar Pradesh, Jharkhand, West Bengal, Assam, and Odisha, presents a unique combination of production constraints: late sowing (post-rice harvest), terminal heat stress during grain filling (March–April), high humidity, and spot blotch pressure. These constraints demand zone-specific breeding solutions rather than simple extrapolation from national programmes. The All India Coordinated Research Project on Wheat and Barley (AICRP-W&B) centre at Sabour, Bihar (then part of Bihar Agricultural College under Rajendra Agricultural University, and now Bihar Agricultural University (BAU), Sabour), was strengthened in 1988. Since then, the breeding programme has been directed towards developing varieties for both rainfed and irrigated conditions across the NEPZ. The mandate of the centre includes breeding high-yielding, disease-resistant wheat varieties for different agro-climatic zones of Bihar; developing early-maturing, terminal heat-tolerant varieties suitable for late sowing; and identifying suitable genotypes for terminal heat and leaf blight tolerance. Terminal heat stress is a major constraint for wheat production in the NEPZ, particularly under late-sown conditions. QTL mapping studies have identified heat tolerance QTLs on chromosomes 2B, 7B, and 7D, associated with Canopy Temperature Depression (CTD), grain weight, and grain-filling duration under heat stress [43]. These reported QTLs provide candidate regions for further validation in NEPZ-adapted germplasm across representative target environments before marker-assisted deployment [43, 86, 87]. These findings highlight the potential for genomics-assisted breeding to address terminal heat stress in the EIGP region.
8.2. Strategic Recommendations
Broadening the genetic base through systematic utilization of landraces, wild relatives, and pre-bred lines in crossing programmes should be prioritized. The primary gene pool provides the most accessible route for introgression of D-genome diversity [27, 29]. This includes Ae. tauschii and synthetic hexaploids in particular. The secondary gene pool (including Triticum timopheevii, Aegilops kotschyi, Ae. variabilis, and Ae. umbellulata), however, harbours unique disease resistance genes, heat tolerance alleles, and drought adaptation traits unavailable in the primary gene pool [28]. The tertiary gene pool includes Thinopyrum elongatum, Th. intermedium, Leymus racemosus, and Agropyron cristatum. It offers genetic material for extreme heat and drought adaptation, FHB resistance, and novel agronomic traits not present in cultivated wheat or its closer relatives. This pool should be systematically explored through structured pre-breeding programmes [27, 28]. Introgression from secondary and tertiary pool species requires chromosome engineering, but multiple successful transfer events have been documented, including the 7Ag.7DL translocation from Th. ponticum carrying the Lr19 leaf rust resistance gene. Developing heat- and drought-tolerant varieties through introgression of adaptive alleles combined with genomic selection represents a high-priority avenue for EIGP-specific breeding. Investment in controlled environment speed breeding facilities, high-throughput genotyping platforms, and drone-based phenotyping infrastructure at SAUs is essential. Continued implementation and clarification of science-based regulatory frameworks for gene-edited crops, building on India's 2022 SDN-1/SDN-2 exemption and drawing on approaches adopted in the USA and Brazil, could facilitate the development and translation of CRISPR-derived wheat varieties in India. Public-private partnerships modelled on those established in the hybrid seed sector should be encouraged to catalyse investment in advanced wheat breeding technologies.
8.3. Future Directions
The future of wheat breeding lies in seamlessly integrating advanced genomic tools, precision phenotyping, and accelerated generation advancement into efficient and cost-effective breeding pipelines. AI and ML methods applied to multi-environment trial data analysis, genomic prediction, and crossing scheme optimization hold significant promise for increasing genetic gain per year [79]. Developing hybrid wheat systems that exploit Cytoplasmic Male Sterility (CMS) and chemical hybridizing agents could further enhance yield potential by capturing heterosis. De novo domestication of wild wheat relatives using CRISPR technology offers a long-term avenue for developing new crop variants combining superior stress tolerance with high yield potential [88]. Systematically harnessing pangenome-level diversity through haplotype-based breeding will be a defining feature of the next generation of wheat improvement programmes.
CONCLUSION
Wheat remains an indispensable crop for global and Indian food security. Its genetic improvement is more urgent than ever, given a rapidly growing population, accelerating climate change, and evolving biotic stresses. This review has synthesized current knowledge across the spectrum of wheat genetics, genomics, and breeding. The completion of the bread wheat reference genome, development of pangenome resources, and the application of genomic selection, speed breeding, GWAS, and CRISPR-based editing have collectively transformed the wheat improvement landscape. Stability analysis frameworks, including the AMMI model and Eberhart–Russell regression, provide essential statistical tools for identifying broadly adapted and specifically adapted genotypes for multi-environment deployment. This capability is particularly critical for the diverse agro-climatic zones of Bihar and the broader EIGP. The integration of multi-omics data, high-throughput phenotyping, and AI-driven analytical methods within a coherent and well-funded national breeding programme will be essential for achieving the yield gains required to sustainably feed India and the world in the coming decades. Institutions such as IARI and ICAR-IIWBR will play a central role in supporting this effort.
AUTHORS’ CONTRIBUTIONS
The authors confirm their contributions to the paper as follows: A.K: Conceptualization, literature review, writing - original draft preparation, revision and editing. M.K: Literature search, data compilation, writing - review and editing. C.K: Literature synthesis, figure preparation, writing - review. S.K: Supervision, validation, and writing - final review and editing. All authors reviewed the results and approved the final version of the manuscript.
LIST OF ABBREVIATIONS
| CBF | = C-repeat Binding Factor |
| CIMMYT | = International Maize and Wheat Improvement Center |
| CSISA | = Cereal Systems Initiative for South Asia |
| DArTseq | = Diversity Arrays Technology Sequencing |
| DNA | = Deoxyribonucleic Acid |
| DREB | = Dehydration-Responsive Element-Binding |
| GIF1 | = GRF-Interacting Factor 1 |
| ICARDA | = International Center for Agricultural Research in the Dry Areas |
| IIWBR | = Indian Institute of Wheat and Barley Research |
| LED | = Light-Emitting Diode |
| NAC | = NAM, ATAF, and CUC transcription factor family |
| PCR | = Polymerase Chain Reaction |
| RFLPs | = Restriction Fragment Length Polymorphisms |
| RGB | = Red-Green-Blue (imaging) |
| RNP | = Ribonucleoprotein |
| SAS | = Statistical Analysis System |
| SPSS | = Statistical Package for the Social Sciences |
ACKNOWLEDGEMENTS
The authors sincerely acknowledge the Department of Genetics and Plant Breeding, Bihar Agricultural University (BAU), Sabour, Bhagalpur, Bihar, for providing the necessary facilities and academic support for this work. This manuscript bears BAU Communication Number 2705/260710. The authors are also grateful to the scientific community and publishers whose valuable works have been cited and reviewed in this manuscript.